Monday, March 19, 2012

Does Air Density Make a Difference?


This is essentially a cross-post from H2VP (with some additions)

One thing I have been asked with some regularity is whether or not a somewhat denser Mesozoic atmosphere, particularly in the Cretaceous (compared to the modern one), could explain the giant size of Late Cretaceous pterosaurs or large dinosaurs.  In short, the answer is: probably not.

There is a reasonably good body of information regarding atmospheric composition during the Mesozoic.  During the Cretaceous, both oxygen and carbon dioxide levels rose slightly, and the total atmospheric density would have been slightly greater as a result - but the difference would have been relatively mild for large vertebrates.

Here is an example of a paper published on the effects of Cretaceous oxygen concentrations on plants: http://jxb.oxfordjournals.org/content/52/357/801.full, and there is a manuscript examining the effect of paleoatmosphere conditions on insects: http://jeb.biologists.org/content/201/8/1043.full.pdf.  There is a relatively recent paper on the Late Cretaceous atmosphere and its potential relationship to mass extinction as well: http://jxb.oxfordjournals.org/content/52/357/801.full

As you can see, plants and insects probably felt the effects of slightly higher oxygen and carbon dioxide concentrations, and indeed the insects of the Cretaceous included some relatively large species, as would be expected.  A slight increase in atmospheric density would have relatively little impact on the maximum size of dinosaurs or pterosaurs, however, and there is not actually any need for an extreme explanation for their size, anyway - despite being larger than living animals with similar lifestyles, none of the giant dinosaurs exceeded the expected maximum size for a walking animal, and no pterosaurs exceeded the limits for biological flight.  Quite a few pterosaurs exceeded the estimated limit for continuous flapping flight in a vertebrate animal (limit is roughly 25-30 kg, give or take), but that only means that they could not flap continuously over long distances and would have switched to soaring flight for long trips; it does not forbid them from flying.

There are three reasons why changes in atmospheric conditions have greater impacts on insects than vertebrate flyers.  First, the tracheal system that insects use for respiration is highly sensitive to oxygen partial pressure.  Second, since insects are typically small, they are often highly reliant on unsteady aerodynamics, which are much more sensitive to air density than steady dynamics.  Finally, insects are almost purely aerobic flyers, while many vertebrates can utilize some degree of anaerobic power (in large flying vertebrates, anaerobic power dominates).  Using anaerobic flight muscle provides a very large burst of power, without using oxygen, after which the muscle quickly fatigues.  Large vertebrates can therefore flap for short bursts, followed by periods of gliding, even when oxygen levels are low.  This option is typically unavailable to insects.

Thursday, March 15, 2012

Looking for the lost

Over on the Archosaur Musings I have a post up asking for help in finding all of the various 'missing' pterosaurs from the Solnhofen. In short, specimens which are out there but are not recorded in the literature. For simplicity, I've reproduced the whole post below, but if you know of any please post them over on the Musings as it's much easier for me to keep track of things there and already there are some reports coming in which is good to hear.

......................................

There have recently been a number of papers describing 'lost' or little known pterosaurs from around the world. I've covered the Rhamphorhynchus that sat undescribed in Dublin for over a century, and I've mentioned specimens on display in Japan that have never been in the literature. There are others too that are starting to come out, like a Pterodactylus in France and others in Hungary. While obviously some of these are making it into the literature, there are others that haven't (like those in Tokyo and I know of one in Kiel) and I'm most interested in finding them.

There's an obvious reason for this - completeness. While Peter Wellnhofer did a great job in the 70s of collating Solnhofen specimens and measurements in two major papers, a lot of time has passed since. New material has been discovered, and old material has come to light. I'm sure there's a significant number of specimens now out there available for study that are either not in the literature at all, or are only mentioned or illustrated and have no good descriptions or measurements put down.

These are of course well worth knowing about. Pterosaurs remain rare and history alone means that the Solnhofen is the best studied and best known set of pterosaur fossils going. Combined with the presence of both pterodactyloids and more basal forms, and generally large numbers of good quality material it is perhaps our premier source of data right now. As such knowing what we have and maximising this is important for science and can allow us to do bigger and better analyses, or sort through what we have and select specimens that can be sacrificed for sampling or are worthy of further attention and preparation.

In my experience many of these 'lost' specimens are often on display, right there and easy to see (as pterosaurs are rare and often a prime piece worthy of exhibition). Provided of course you are in the museum to see them! The Kiel specimen I mentioned was one such - to my knowledge or that of any of my colleagues I'd spoken too, they simply didn't have any Solnhofen material at all, none. So a pterosaur expert is rather unlikely to there to check out a tiny palaeontological collection which shouldn't contain anything of interest and let's face it, there's a lot of museums out there.

Bearing that in mind, if you do come across a Solnhofen pterosaur in an odd and usual place (i.e. not the Carengie, or London NHM or the like) do please let me know. Sure it might turn out to be a cast, or even a well-known specimen, but the number that are increasingly coming out of the woodwork make me suspect there's rather more out there and it would be great to try and track them all down and one day get them into the formal literature. If you have a photo or specimen number, even better, but a simple mention of what you saw in which museum would be a great start. I'm convinced there's a significant number of specimens out there and they are well worth finding.

Monday, March 12, 2012

Talk at the Royal Tyrrell Museum

Last week, I gave a pterosaur talk at the world famous Royal Tyrrell Museum, in Alberta, Canada.  The museum has its own YouTube Channel and has made my talk freely available here:

http://youtu.be/5wmds4zq5Eg

They also have a series of previous talks by other researchers recorded and available.

Cheers,

--MBH


Saturday, February 25, 2012

Staking the vampire pterosaur: Jeholopterus was NOT a vampire


It's a common misconception that staking the heart of a Stokerian vampire will do it in for good. In actuality, the characters of Bram Stoker's Dracula (above) only considered the undead truly out of action once they were staked through the heart (which only imobilised them, see, not killing them), decapitated, had their mouths stuffed with garlic flowers and the access to their tombs lined with holy masonry. This may seem like overkill, but, for the vampire mythos Stoker created, it is the only way to keep the blaggards down. In the last week, it's emerged that that palaeontological vampires need a similar heavy duty approach to ensure that they too don't continue to rise from the grave.

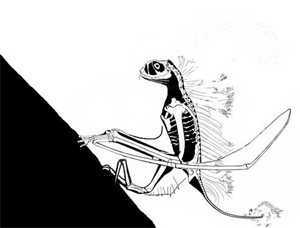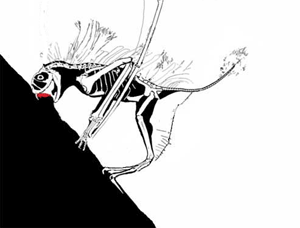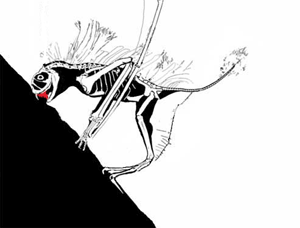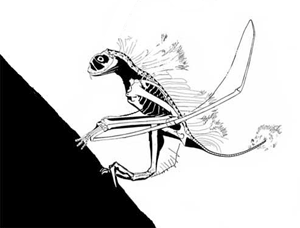
LinkEnter, stage left, the hypothesis that the anuroganthid Jeholopterus was a Mesozoic vampire bat equivalent (image, above, from my upcoming book, shows the anuroganthid Anurognathus with a more accurate Insect Hawking Cookie Monster of Doom appearance, not a vampire). Proposed by David Peters in an abstract for the SVP annual conference of 2003, cited evidence for this idea stems from large caniform teeth inferred on the Jeholopterus holotype using DP's infamous digital photo interpretation (for anyone unfamilar with DP's work, you can see the most recent incarnation of it here). It is well known that palaeontologists have almost never seen eye to eye with Peters' interpretations of fossils or methods of analysing them, and a small body of literature exists that directly refutes his work (e.g. Bennett 2005; Hone et al. 2009) . Many other papers also disagree with his methods or conclusions. DP acknowledges his 'heretical' views and, indeed, has even named his blog after them: The Pterosaur Heresies. Our very own Pterosaur.Net even gets a good kicking at various points at TPH, but that's OK: we have our opinions (which we consider to be well supported and credible), and Dave has his (which we consider to be very poorly supported). I think we have to live with the fact that we're not going to agree with everyone in science, and, frustrating though this can be at times, we're much better off making sure our own work is as watertight as possible than constantly bickering with others.

The vampire Jeholopterus made a brief splash back in 2003, but was widely condemned by the entire pterosaur community. To many, this simply proved - again - that SVP perhaps needed to pay closer attention to the work they were allowing into their conference, but that was that. No peer reviewed paper on the vampire hypothesis followed, and no independent confirmation that Jeholopterus or other anurognathids were sanguivorous has been proposed. Instead, the long-held view that anurognathids were ace aerial insect hawkers has prevailed (e.g. Bennett 2007; Habib 2011 [a follow up publication to which is in the works. I'm lucky enough to have been invited in on the authorship and can promise that some of the stuff in it should blow your little socks off]). The vampire pterosaur idea, it seemed, was dead, the only remnants being the abstract, a few media stories, and the Jeholopterus page at DP's website. This week, however, the vampire Jeholopterus meme has risen from the grave, being portrayed in a half-credible light in this article and picked up elsewhere online. Several people, including myself, were a bit miffed at this, and, in full on SIWOTI mode, left comments on these articles. The original article seems to be picking comments that agree with the tone of the article as their 'featured' comments, hiding perhaps more informed opinions in other pages of the article. Hence, seeing as most people won't easily find these remarks, I thought best to regurgitate mine here. In short, I want to provide a one-stop shop for clarity on the vampire pterosaur hypothesis:

  • The idea was not peer reviewed, and it's publication in a collection of conference abstracts is not of comparable standing to other hypotheses of anurognathid palaeoecology
  • There was never any 'debate' amongst pterosaur workers on this idea: it was never considered credible by qualified researchers in the first instance, and rejected outright from the start.
  • There is no evidence that Jeholopterus, or any other pterosaur, was a vampire
  • There is no 'David Peters vs. Goliath' story here. DP's work is considered with the same scrutiny, not more or less, than any other piece of science. His ideas are rejected by other palaeontologists (amateur and professional alike, the only difference between many of whom is that some are paid to study fossils) because they have not stood up to this scrutiny.
Any claims to the contrary suggest very lazy journalism, I'm afraid, so shame on those who have given this idea even a whiff of credibility. With that, I'll hand you over to my rambly self of yesterday, when I commented on the article that inspired this post. Said article may make for required reading before you continue.

--

This story has been told rather incorrectly. DP's 'publication' in 'the peer-reviewed Journal of Vertebrate Paleontology' was NOT peer reviewed: it was a short abstract for the SVP 2003 annual conference. I am confident as a 'professional' pterosaur worker myself that this paper would not have made it into any scientific journal, and it was rightly condemned by the pterosaur community as soon as it was made public. Along with the Bennett article mentioned here, a body of literature exists demonstrating that most, if not all, of David Peter's methods of reconstruction and image interpretation are flawed. The extraneous features he reconstructs for fossil animals (which have included, at one time or another, fantastic frills, sails, additional bones and teeth, long tails on short-tailed taxa, hatchlings clinging to their parent's body and others) have never been found on fossil specimens despite CT scanning, UV investigation and other analytical methods. The vast majority of DP's ideas are not corroborated by any studies except his own. In polite terms, DP's ideas are considered 'fringe' at best by palaeontologists, and very much the view of one individual. (animated vampire Jeholopterus feeding strategy, below)


I find it worrying that you wrote your article without uncovering or featuring these details. Likewise, the fact that you give the vampire Jeholopterus idea some credence with statements like 'what spurred the great debate' and 'without a living Jeholopterus to observe, we really cannot be sure of its unique attributes': there was never any debate, and the latter suggests a critical misunderstanding of scientific practise. Palaeontologists work, like all other sciences, by testing hypotheses: we are confident that Jeholopterus was not a vampire bat-like animal because it fails tests we can put against this idea. Does it bear large teeth for piercing flesh? No. None have ever been found on any actual specimen: the fact they have been found on someone's computer screen means nothing if they cannot be seen by some means on the actual fossil. DP probably picked up compression artefacts in the jpeg or cracks, shadows and prep marks in the matrix on the slab. Did Jeholopterus have a strong bite? Probably not, as the bones of the jaw are mechanically weak and slender, and ill-suited to anchoring strong muscles. Are there any alternative means it could use to pursue a vampire lifestyle? None that we can ascertain. Is there a more plausible hypothesis for the lifestyle of Jeholopterus? Yes: aerial insectivory, a lifestyle that decades of _actual_ peer-reviewed studies into anurognathid (the group that Jeholopterus belongs to) anatomy and biomechanics support without exception.

Finally, the portrayal of DP as a maverick, lone amateur 'informing' the body of professional palaeontologists is unfair. A great number of so-called 'amateur' palaeontologists produce work of the highest credibility without a whiff of controversy. Like DP, they work alone and draw their own conclusions, but find that their ideas are similar to those lucky enough to be paid to research palaeontological subjects. There is no conspiracy about preservation of dogmatic ideas or rejection of outsiders: the internet teems with blogs and forums where paid palaeontologists and 'amateuers' meet to discuss ideas at the highest level. I'm afraid to say I find this article very ill-informed and misleading, and hope this comment adds some balance to this page.

References

  • Bennett, S. C. 2005. Pterosaur science or pterosaur fantasy? Prehistoric Times, 70, 21-23.
  • Bennett, S. C. 2007. A second specimen of the pterosaur Anurognathus ammoni. Paläontologische Zeitschrift, 81, 376-398.
  • Habib, M. B. 2011. Functional morphology of anurognathid pterosaurs. Geological Society of America Abstracts with Programs, 43, 118.
  • Hone, D. W. E., Sullivan, C. and Bennett S. C. 2009. Interpreting the autopodia of tetrapods: interphalangeal lines hinge on too many assumptions. Historical Biology, 21, 67-77.
  • Peters, D. 2003. The Chinese vampire and other overlooked pterosaur ptreasures. Journal of Vertebrate Paleontology, 23(3), 87A.

Sunday, February 12, 2012

The top 5 most important pterosaur specimens

As usual when it's me on here, this is a repost from my blog. Still, if ever I wrote something that was made for Pterosaur.net this was it. So, here is something that does rather combine every aspect of pterosaur research into one neat package.


Just an idle bit of fun this, but the thought was running through my head and I thought there was a blog post in there somewhere so decided to have a go at it. All very subjective of course and hard to assess but there are issues of completeness, importance, the scientific information held or conveyed by the material and other things. Anywhere, here’s my effort at least (in no particular order):

1. The Dark Wing Rhamphorhynchus.

Specimens from the Solnhofen are not uniquely flat, but the vast majority are compressed into two dimensions. The sheer number of Rhamphorhynchus specimens means that we do have a great understanding of their anatomy and ontogeny, even if it is 2D and there are lots of specimens with bits of soft tissues or unusual details preserving. This specimen though pretty much has it all. It’s complete, the bones are nearly entirely in 3D and it comes with a magnificently preserved set of wing membranes – easily the best out there. Stick all that together and it’s a hell of a specimen.

2. Jeholopterus holotype

Sure Sordes is nice and already covered in pycnofibers, but Jeholopterus is much the better preserved with more details of both ptero-fuzz and the wings. As a bonus it’s by far the best preserved anuroganthid specimen (well in total, the juvenile Anuroganthus is magnificent but has no softs), an otherwise badly known but potentially very important group.

3. The Tokyo Anhanguera

Probably the single most complete and 3D specimen I know of. Sure there are a few bits missing, but unlike the dark-wing, every bone is free of the matrix and can be picked up, turned around, examined from every angle and checked. Sadly it’s a juvenile and so some of the features aren’t quite what they would be at adult, but it is one hell of a specimen for the actual gross skeletal anatomy.

4. The Darwinopterus + egg combo

This one is a bit fortuitious since it does rather let me get a two-for-one with both a transitional pterosaur (and just how significant that is for a number of reasons) and gives us a bona fide pterosaur egg. Each tells us so much about pterosaurs and pterosaur evolution, it’s an incredible animal.

5. The big Quetzalcoatlus.

Every specimen can tell you something, and there are surprises everywhere. The new Nyctosaurus and Thalassodromeus revealed how huge crests could get, the series of ‘Tapejara’s told us about the integration of soft tissues, Raeticodactylus served a warning about eudimorphodontid-like teeth for taxonomy. But head and shoulders over all of this is the giant specimen of Quetzalcoatlus (even if it isn’t yet properly described). Size is such a crucial aspect of the biology of any organism, but in this case it is simply so big and in a flying animal too, that it really was almost a gamechanger for our understanding of pterosaurs in their own right. That a flying animal could get this big was a shock (despite some of the wild estimates, 10 m is bloody massive!).

And to close out, a few near misses from the list: footprints that showed us how they walked, the Pterodactylus holotype which brought pterosaurs to the world, one of the embryos which proved they did lay eggs and gave us a window into their life history.

Monday, February 6, 2012

Tapejara wellnhoferi: the lost reconstructions

Ross A. Elgin

Only twenty three years after it was formally named Tapejara wellnhoferi [1], one of the best known azhdarchoids from the Araripe Basin of NE Brazil, finally has a body! While, if I’m honest, this isn’t exactly new news, the original publication being released in the Swiss Journal of Palaeontology by my colleague Kristina Eck towards the end of last year [2], there is at least some merit to a post looking back at this particular discovery.

For a start, in case you missed it the first time around, the specimen is very unusual in that the remains of two juvenile pterosaurs – one largely complete and one represented by a partial wing, became embedded together within a single nodule. To the best of my knowledge the original concretion thus represents the only example of a multiple death assemblage in pterosaurs where neither specimen has been reworked from another layer of strata; a factor almost certainly attributable to the low preservation potential of the pterosaurian skeleton coupled with the presumably large geographical distance throughout which these animals were capable of being dispersed. Whether this unusual taphonomy was brought about by two unlucky individuals being downed during a storm, swept in from a nearby nesting site or simply as a result of local water currents, however, remains very much an open and unanswerable question.

Although numerous azhdarchoid postcrania are known the Early Cretaceous of Brazil they are almost always indeterminate owing to the lack of the skull and so remain of limited taxonomic value (to the great frustration of both myself and I’m sure other palaeontologists working on these animals). With this in mind the most valuable information that these two individuals are able to provide is a detailed look at the postcranial skeleton in a species so often defined solely by its cranial remains, and based on this the first reconstruction of T. wellnhoferi is presented here. The reconstructions posted below were originally destined to be included with the original description, however, were unfortunately cut due to space restrictions in what was an already overly long research paper. While it is thus worth noting that these diagrams have not been reviewed by the wider scientific community I nonetheless feel it best to present them here for reference and the benefit of future researchers or other interested parties.


Figure 1. Tapejara wellnhoferi reconstructed from skeletal material of SMNK PAL 1137 in left lateral view. Forearm and tibia/pes omitted for clarity. Bones shaded in grey indicate preserved elements.


Figure 2. Tapejara wellnhoferi reconstructed from skeletal material of SMNK PAL 1137 in ventral view. Bones shaded in grey indicate preserved elements. Left side of the body omitted to increase visibility.

So there we have it, in addition to some nice notes on the endocranial cavity and pneumatic system, for which I don’t have space to delve into here, Tapejara wellnhoferi finally gets its body and we can all enjoy a long awaited reconstruction of the animal, along with some interesting thoughts on pterosaurian taphonomy.

References

1. Kellner, A. W. A. 1989. A new edentate pterosaur of the Lower Cretaceous from the Araripe Basin, Northeast Brazil. Anais de Academia Brasileira de Ciencias 61:439-446

2. Eck, K., Elgin, R.A., Frey, E. 2011. On the osteology of Tapejara wellnhoferi KELLNER 1989 and the first occurrence of a multiple specimen assemblage from the Santana Formation, Araripe Basin, NE-Brazil. Swiss Journal of Palaeontology, doi: 10.1007/s13358-011-0024-5.

Sunday, January 8, 2012

Pterosaur.net research 2011

About this time last year I put together a little post about all the work that had been done by various members of the P.net team over the previous 12 months. Obviously we continue to carry out and publish research and are involved in conferences and the like. I thought it fun to carry on with this pattern, so here is what we've put together from 2011. It's rather less than last year quite simply because we'd had the Flugsaurier meeting in Beijing which naturally resulted in an additional glut of abstracts. Even so there's a good mixture of conference material and real research papers here and it covers quite a range of pterosaur subject including flight, ecology, taxonomy, anatomy and even history of research.

Here's to the pterosaurs of 2012.


Andres, B., Howard, L., & Steel, L. 2011. Owen’s pterosaurs, old fossils shedding light on new clads. Symposium for Vertebrate Palaeontology and Comparative Anatomy (SVPCA), Lyme Regis, UK.

Chapman, S. & Steel, L. 2011. Reptiles from the Lower Lias of the Dorset Coast and Mary Anning. Symposium for Vertebrate Palaeontology and Comparative Anatomy (SVPCA), Lyme Regis, UK.

K. Eck, R.A. Elgin & E. Frey. On the osteology of Tapejara wellnhoferi KELLNER 1989 and the first occurrence of a multiple specimen assemblage from the Santana Formation, Araripe Basin, NE-Brazil. Swiss Journal of Palaeontology, DOI: 10.1007/s13358-011-0024-5

Elgin, R.A., & H.B.N. Campos. A new specimen of the azhdarchoid pterosaur Tapejara wellnhoferi. Historical Biology, DOI: 10.1080/08912963.2011.613467

Elgin, R.A., & E. Frey. A new ornithocheirid, Barbosania gracilirostris gen. et sp. nov. (Pterosauria, Pterodactyloidea) from the Santana Formation (Cretaceous) of NE Brazil. Swiss Journal of Palaeontology, DOI: 10.1007/s13358-011-0017-4

Elgin, R.A., & E. Frey. A nearly complete ornithocheirid pterosaur from the Crato Formation (Aptian, Early Cretaceous) of NE Brazil. Acta Palaeontologica Polonica DOI:10.4202/app.2010.0079

Elgin & E. Frey. A new azhdarchoid pterosaur from the Cenomanian (Late Cretaceous) of Lebanon. Swiss Journal of Geoscience, DOI: 10.1007/s00015-011-0081-1

*Elgin, R.A., Hone, D.W.E. & Frey, E. 2011. The extent of the pterosaur flight membrane. Acta Palaeontologica Polonica, 56: 99-111.

Habib, M. 2011. Functional Morphology of Anurognathid Pterosaurs. GSA Northeast Regional Conference •2011.

Habib, M. Solving the pterosaur size problem: Quadrupedal launch in the Pterosauria. Los Angeles County Museum

Hone, D.W.E., Naish, D. & Cuthill, I.C. Cranial ornamentation and sexual selection in pterosaurs and non-avian dinosaurs. Lethaia, in press.

Hone, D.W.E. A new specimen of the pterosaur Rhamphorhynchus. Historical Biology, in press.

Hone, D.W.E., Henderson, D.M. & Palmer, C. 2011. Investigating the buoyancy and floating posture of pterosaurs. Symposium for Vertebrate Palaeontology and Comparative Anatomy (SVPCA), Lyme Regis, UK.

Lawlor, E., Beardmore, S., Hone, D.W.E., & Orr, P. 2011. Skeletal taphonomy of pterosaurs from the Late Jurassic of Germany. Symposium for Vertebrate Palaeontology and Comparative Anatomy (SVPCA), Lyme Regis, UK.

Sweetman, S.C., Martill, D.M. & Witton, M.P. 2011. Pterosaurs. In
Batten, D.J. (ed.). English Wealden fossils. Palaeontological
Association, London, Field Guide to Fossils, 14, 769 pp.

Witton, M.P. 2011. The pectoral girdle of Dimorphodon macronyx
(Pterosauria, Dimorphodontidae) and the terrestrial abilities of
non-pterodactyloid pterosaurs. SVPCA 2011 Programme & Abstracts, Lyme
Regis, 2011, 22.

Witton, M.P. & Maclean-Henry, G. 2011. Additional details on the
skull of Istiodactylus latidens and the palaeoecology of istiodactylid
pterosaurs. SVPCA 2011 Programme & Abstracts, Lyme Regis, 2011, 28.

*Came out in 2010 and we talked about it then but, well, it does have a 2011 date on it.